Showing posts with label mysticeti. Show all posts

Thursday, August 9, 2012

Parabalaenoptera baulinensis: the fossil baleen whale from Bolinas, Marin County, California


Until relatively recently, fossil balaenopterids have been avoided by modern paleocetologists like the plague. Modern balaenopterids include the humpback whale (Megaptera novaeangliae) and species of Balaenoptera, including the Minke, Blue, Fin, and Sei whales. Although balaenopterids have very distinctive and easy to identify crania, they are really only common in latest Miocene and Pliocene marine rocks, and early work by Kellogg and others yielded fossil baleen whales with much more primitive skulls, formerly called "cetotheres" sensu lato, also jokingly referred to by some paleocetologists as "Kelloggitheres".

Fossil balaenopterids have been plagued by a particularly nasty taxonomic situation since the late nineteenth century, when P.J. Van Beneden began describing fossil mysticetes collected during the construction of a series of forts around Antwerp. Unfortunately, many of these fossils which names like Plesiocetus and Herpetocetus are based upon were isolated finds, which were subsequently arranged into type 'series' with other skeletal parts based on a preconceived notion of what each taxon should have looked like. The end result was a series of chimaeras, some of which represented by potentially informative but often fragmentary material, lacking type specimens, the associated names of which have been dragged through the systematic mud by subsequent authors, and not allowed to simply die gracefully.

The skull and mandibles of the holotype specimen of Parabalaenoptera baulinensis from the late Miocene Santa Cruz Mudstone of Marin County, California.

Many of these fossil balaenopterids are difficult or impossible to diagnose: which specimen of the series would you designate as a lectotype? Is that specimen diagnostic? What do you do with the other specimens? Is an isolated mandible diagnostic or not? What about a piece of a braincase with unassociated bullae? According to Bosselaers and Post (2010), many of Van Beneden's taxa are based on "syntype" collections that are not possible to unambiguously diagnose: diagnostic syntype elements are either too incomplete, or include multiple diagnostic elements but from multiple individuals (and occasionally taxa; i.e. a balaenid bulla was grouped with the lectotype mandible of Herpetocetus scaldiensis by Van Beneden). Accordingly, Bosselaers and Post (2010) declared all of Van Beneden's Pliocene balaenopterid taxa to be nomina dubia: for the time being, I think this is probably the "safe", appropriate, and right thing to do.

The discovery and description of Parabalaenoptera baulinensis was one of the first important advances in balaenopterid paleontology: it was one of the first balaenopterids described from a nearly complete skull with associated mandibles and postcrania. Some other previously published fossil balaenopterids were described on somewhat complete remains: Megaptera miocaena (late Miocene of California), Megaptera hubachi (late Miocene of Chile), Protororqualus cortesii (Pliocene of Italy), "Balaenoptera" cortesi var. portisi (Pliocene of Italy), and Cetotheriophanes capellinii (...also Pliocene of Italy). Unfortunately, the holotype skeleton of Protororqualus was destroyed during bombing in World War II, and M. miocaena only includes earbones and a braincase; furthermore, the other Italian balaenopterids have been plagued with nomenclatural issues for over a century (see Demere et al. 2005).
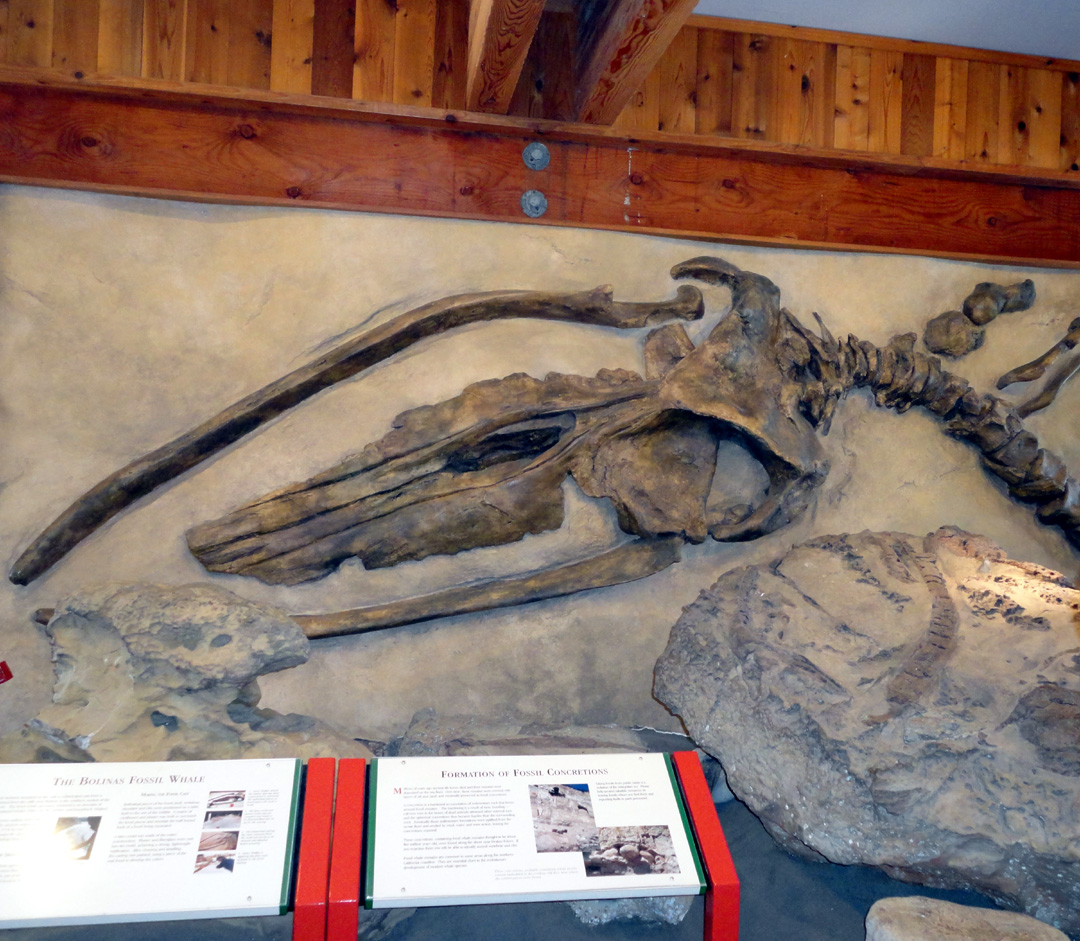
The exhibit at the Drakes Beach visitor's center showing the holotype skeleton of 
Parabalaenoptera baulinensis.

In 1973, a large mysticete skeleton was discovered by Carl Zeigler of the College of Marin, weathering out of cliffs near Bolinas in Marin County, California. Bolinas is a quaint artist community on the Marin County coast and has changed little since the 1960's and 70's; it is predominantly settled by ex-hippies, who generally don't like visitors from out of county, and have continually removed the exit sign for "Bolinas: 2 miles" off of highway 1, to the point where the California Dept. of Transportation (CalTrans) has given up putting up new signs. Tales abound of visitors with out of county or out of state license plates having car tires popped or vandalized, and nails and other tire-popping objects being intentionally laid out onto dirt roads in town. My car had a San Rafael Honda license plate holder, so I never had this problem.

The assembled holotype skull of Parabalaenoptera at California Academy of Sciences, photographed by fellow Otago Ph.D. student Felix Marx.

Exposed along the southern tip of Point Reyes is a unit formerly identified as the early late Miocene Monterey Formation; this was subsequently reevaluated after Domning (1978) suggested that sea cow fossils from the Bolinas locality were too derived to be from such an old unit. Afterwards, microfossils suggested a much younger age, closer to the Mio-Pliocene boundary (6-6.8 Million years old), and the formation was reidentified as the Santa Cruz Mudstone, which has only been mapped in Santa Cruz County.

Anterior view of Parabalaenoptera.
The fossil occurred in indurated, blocky mudstone, and was collected over a ten year period as the blocks incrementally eroded from the cliff. The lead authors - Gordon ("Gordie") Chan and Carl Zeigler of the College of Marin in Kentfield, and their field assistants - would have to travel over the hill and out to Bolinas (nearly an hour's drive through some of the windiest vomit-inducing roads in Northern California) on a monthly basis during the summer, and much more often during the winter during periods of intense erosion, and sometimes daily, anticipating falling blocks. After collection, the blocks were prepared, and some were glued together - but left as a series of blocks that could be lined up and assembled. The holotype was prepared at College of Marin, and eventually molded, casted, and donated to the California Academy of Sciences. Mounted casts of Parabalaenoptera baulinensis are currently on display at College of Marin in Kentfield and at the Drake's Beach visitor center at Point Reyes National Seashore. Sadly, before the paper could be published on the fossil - Carl Zeigler and Gordon Chan passed away. Chan passed away in 1996 of Lou Gehrig's disease; I could not find information on Zeigler, though I seem to recall hearing that he was killed by a drunk driver. Dr. Lawrence Barnes of the Los Angeles County Museum of Natural History finished the manuscript and brought it to publication in the California Academy of Sciences in 1997.

The braincase and vertex of Parabalaenoptera.
Parabalaenoptera baulinensis is a medium-sized balaenopterid with a 2.2 meter skull, slightly larger than minke whales (Balaenoptera acutorostrata; a 10 meter long whale with a 2m skull), but has a number of features that are too divergent to warrant inclusion within humpbacks (Megaptera) or Balaenoptera. These include the very elongate and somewhat swollen zygomatic processes, narrow intertemporal region (the skull is less 'telescoped than in modern balaenopterids), and extremely long and narrow nasal bones. The mandibles are strongly outwardly bowed like in Megaptera, and have an elongate coronoid process - somewhat like blue and fin whales (Balaenoptera musculus and physalus). Many of these features suggest that Parabalaenoptera baulinensis was capable of lunge feeding just like modern rorquals. It is additionally convergent with Balaenoptera musculus in having a supraorbital process of the frontal that is somewhat triangular and narrows laterally, whereas in Balaenoptera and Megaptera, the posterior and anterior margins are either parallel, or the posterior margin is perpendicular to the midline. Unfortunately, the holotype specimen is not preserved very well, and it appears that a significant amount of bone was accidentally removed or ground away during preparation, and details of the basicranium are almost totally indiscernible. Parabalaenoptera has been found in many phylogenetic analyses to be a stem-balaenopterid - in other words, a primitive member of the clade (family Balaenopteridae) that does not belong to the clade formed by humpback whales and modern species of Balaenoptera - the Megaptera + Balaenoptera clade, if you will. These two modern genera have been traditionally grouped into the "Megapterinae" and "Balaenopterinae" - Zeigler et al. (1997) even went so far as to name a new subfamily, the Parabalaenopterinae. However, given that none of these subfamilies have really shown to be stable or even consistent in cladistic analyses, it's unclear what the utility of such taxon names even is.

Reconstruction of the holotype skull and mandibles of Parabalaenoptera. Unfortunately, certain features (e.g. squamosal morphology) of the actual skull don't really look like how they're portrayed in this figure. From Zeigler et al. (1997).

Nevertheless, the description of Parabalaenoptera was a hallmark in balaenopterid paleontology; however, given the stagnated taxonomic situation of fossil balaenopterids, little else was published on fossil balaenopterids until Michelangelo Bisconti started revisiting Italian fossils starting in 2007. In the last five years, a number of informative balaenopterid finds have been described - but it is only the tip of the iceberg. Perusing late Miocene and Pliocene marine mammal assemblages in Museums, it is apparent that balaenopterids comprise nearly two-thirds of the more recent baleen whale fossil record (it is at least the case for California marine mammal assemblages). In California, at least four to five unpublished balaenopterids await description from the Pliocene alone. Additional fossils that may represent Parabalaenoptera - potentially a new and slightly younger species - have been collected from the Purisima Formation near Santa Cruz (and are in much better condition than the holotype). The future of balaenopterid paleontology is bright!

References

Bosselaers, M., and Post, K. 2010. — A new fossil rorqual (Mammalia, Cetacea, Balaenopteridae) from the Early Pliocene of the North Sea, with a review of the rorqual species described by Owen and Van Beneden. Geodiversitas 32:331-363. 

Deméré, T. A., Berta, A., and McGowen, M. R. 2005. — The taxonomic and evolutionary history of modern balaenopteroid mysticetes. Journal of Mammalian Evolution 12:99-143.


Domning, D. P. 1978. — Sirenian evolution in the North Pacific Ocean. University of California Publications in Geological Sciences 18:1-176.


Zeigler, C. V., Chan, G. L., and Barnes, L. G. 1997. — A new late Miocene balaenopterid whale (Cetacea: Mysticeti), Parabalaenoptera baulinensis, (new genus and species) from the Santa Cruz Mudstone, Point Reyes Peninsula, California. Proceedings of the California Academy of Sciences 50(4):115-138.


Thursday, April 5, 2012

Visit to the Otago Museum

I know there are some readers of this blog who have patiently waited and waited for pictures of beautiful Oligocene marine mammal fossils - to you I say, sorry for the delay. I'm going to try and get several blog posts written this weekend so I can post them incrementally. This one will mostly be in 'slideshow' format.

I've been fairly busy since I got here, and I've bordered on stress trying to figure out 1) where all the eomysticetid specimens are in collections, 2) which earbones belong to which skull or skeleton (just taking a while to become familiarized with the specimen numbers), 3) trying to make some sense out of the earbones and trying to group them based on consistently seen characteristics (and I have made a bit of headway), and 4) just generally trying to figure out how many taxa I am dealing with and thus 5) how many manuscripts/dissertation chapters this will end up making. Since I've finally made some headway and started describing the first material (a partial skull with earbones and a very partial postcranial skeleton), I've relaxed a bit and can allocate time to other activities. That being said, I'm also locked out of the building for four days due to construction/maintenance activities in the building. Fortunately, this will give me an opportunity to divert some time to my Pelagiarctos study with Morgan Churchill. Also, in other news - I finally finished up my massive manuscript describing an entire marine mammal assemblage from a locality in the Purisima Formation, which resulted in being just over 200 double spaced pages long with 45 figures; Felix Marx graciously offered to take a look, as did Ewan Fordyce. I have a bit of work left cleaning up some figures, but it should be submittable soon.
A spectacularly beautiful dalpiazinid dolphin! Look at those damn teeth! There's another specimen with even crazier incisors, and a full dentition, and jaw.

An archaic edentulous mysticete which may fall somewhere on the cetacean family tree near eomysticetids. This specimen will be part of my dissertation.


The holotype skeleton of the giant moonfish Megalampris keyesi. This set of slabs is seriously about 15 feet long and about 8 feet wide. Described by Gottfried et al. 2006.

A disarticulated skeleton of a squalodelphinid dolphin. My labmate and office mate Yoshi Tanaka is studying squalodelphinids for his dissertation (although their skulls are in better shape than in this specimen).
A partial skeleton of the giant shark Carcharocles angustidens, described by Gottfried and Fordyce (2001). Believe it or not, this specimen was found above the dolphin and moonfish skeletons in the same quarry; the shark was found first, and underneath they ran into dolphin bones; below that, they started seeing fish bones (from what turned out to be a truly monstrous fish). They called the shark Carcharodon angustidens instead, as Mike Gottfried is in the Carcharodon camp; that's fine, we all get along pretty well. Mike will be visiting University of Otago for paleo research in May, which will be a great opportunity to catch up.
Detail of the big, beautiful teeth of Carcharocles angustidens.

Beautiful jaw fragment of the undescribed squalodelphinid from the block photographed above.

The skull of the "Shag Point Plesiosaur", now known as Kaiwhekea. That's pronounced "Ky-feh-key-uh"; one Maori pronunciation is "wh" as an 'f'.

The holotype skeleton of Kaiwhekea; yes folks, that's all one gigantic concretion that is ~20 feet long. It took a crew of 3-6 to collect those blocks over the course of a month (each day).

More photos will be coming soon!

Tuesday, November 15, 2011

New mysticete excavation, part 2

On day two, we returned to continue the excavation process. We had mostly pedestaled the specimen on the first day, but we had not yet undercut the block. We thought we could get all of it out in one large jacket. Unfortunately, I knew this might be difficult because there were multiple fractures through the concretion - most concretions I've collected are very strong and have no cracks, but occasionally large ones are fractured, which could spell disaster during the jacketing process.

The skull on friday morning.

The tunnel I dug under the right side of the skull.

We got back to the locality on friday morning, and began to undercut the pedestal. Normally, a small jacket just requires a trench to be dug around the fossil, and then you undercut the bottom of the trench and dig under the fossil a bit - this allows a lip to be made on the bottom of the fossil with the plaster jacket, ensuring that the entire piece of rock (fossil included) leaves the excavation pit when you flip the jacket over. I've heard horror stories of jacket flipping where a stream of bone fragments pours out of the bottom of the jacket upon removal, and fortunately, this has never really happened to me. On larger specimens such as this, it is routine to dig a tunnel underneath part of it, to ensure that the jacket removes a cohesive block rather than half of it. So, I started doing this, digging from both sides, and after about an hour or so I had a cute tunnel underneath the skull where some strips of burlap could go when it came time to jacketing.

The fossil with dampened paper towel and after application of the jacket.

Late in the day on friday, we finally got to the jacketing process. In all honesty, I had not expected to get to start the jacket until saturday morning - we had scheduled a State Parks ranger to drive by on Sunday at 3pm for jacket pick up, so we knew we had until then. We finished up the plaster jacket right before dinner time.

The jacket right after flipping it.

On saturday morning, we quickly moved to undercut the rest of the jacket, "pop" it, and flip it over. This was particularly hairy, because there wasn't exactly any room to flip the jacket - usually you flip the jacket over, and have ample space to let it rotate along whatever surface you have available, which in paleontology fieldwork, is usually the ground. In our case, sure -we had opened up a large shelf we had dug out, but the fossil was already precariously positioned above a ten foot drop to the beach, more than enough distance for the fossil to break into many pieces if it were to fall. More importantly, if the jacket were to fall off the ledge, it would likely take one of us with it, which would really, really hurt. It would have really helped to have a third person, but we were barely able to lift and flip it between the two of us - we had to lift it and slowly rotate it nearly in place, move it to the side while lifting it, and while Des stayed there holding the jacket up from certain destruction, I ran up and down fetching pieces of wood to wedge it so it wouldn't fall off the ledge. During flipping, some of the fractures inside the concretion opened up, and we could feel the block 'flexing' a little bit. Fortunately, it all stayed together. Unfortunately, there were more bones going back into the cliff, which we will not be able to dig out. There was also a small part of the concretion and a possible bit of the skull left in the cliff, which we will have to return for.

The jacket after the bottom jacket was completed.

Wooden "backbone" for the sand ramp.

After flipping the jacket over, we were able to put on a plaster jacket over the bottom part of the block. Now that the jacket was completed, we had the problem of getting it down. The block appeared to weigh at least three hundred pounds, and was very heavy due to the concretion inside. There was no safe way to lift the skull down - the heaviest of a jacket that two people of my diminutive stature can manage is about 100 lbs (my friend Chris Pirrone and I once spent four hours moving a 100 lb jacket only 200 feet along a Santa Cruz cliff, while partially submerged at first, then up algae covered rocks, and along a 10 foot high, one foot wide ledge over the ocean, and up several eye-level ledges).

One thing I enjoy about paleontology fieldwork is thinking outside the box. I've had conversations with people who would have used some high-tech rope and pulley system which would have probably been a pain to put together and utilize. In my experience, when moving big (but manageable) pieces of rock, it's best to use methods developed by the masters of lugging around big rocks: the ancient Egyptians. Although it was up rather high, I thought "why not just build a big ramp?". To make it faster, we piled up a bunch of logs: sand usually moves to the angle of repose, and we needed something steeper (so we wouldn't end up with a cone of sand with a twenty foot wide imprint). The logs trapped the sand, and we were able to build a steeper ramp.

My wife with the beginning of the sand ramp, pretending it was her idea.

Des, myself, Ash Poust, and Liz Ferrer (clockwise, from upper left) start to
maneuver the block down the incline.

My wife (left, in red), Liz Ferrer (hiding in back), and Ash (white pants)
excavate a bit of the remaining concretion.

It only took us about a half hour to finish the ramp, and once we were done, we climbed up, and started to nudge the plaster jacket. Our friend Ash Poust, who was a friend of ours from MSU and now one of Kevin Padian's Ph.D. students at UC Berkeley, had brought along another one of Padian's students, Liz Ferrer, to help out. My wife sat out on this one, and took photos instead, while the rest of us muscled the jacket down. It worked like a charm, and I could not have been happier with my experiment in 'ancient methods'.

Stay tuned for the next installment!

Sunday, October 9, 2011

Update: The coastal paleontologist gets married, and goes down under?

The last couple of weeks have been pretty great, and due to being so busy in relation to recent events, I've been a little slow on posting new material on here. First and foremost, I got married to my longtime girlfriend/fiancee Sarah Michalies on September 17 up at beautiful Lake Tahoe, California. The wedding was fantastic, and a lot of fun - and there were many paleontology students from around North America in attendance. Sarah and I have been together since spring 2005, and it was about time to tie the knot. Sarah and I met as undergraduates in the paleontology program at Montana State University, and have gone on all sorts of paleo field trips together.

This is not our boat, we just borrowed it for cool pictures.

The second awesome thing that happened - I was recently (i.e. on Thursday) accepted into the Doctoral program at the University of Otago in New Zealand. I applied back in late July, and the plan is to start in January. I have the fantastic opportunity to work with Dr. R. Ewan Fordyce, who has offered me a chance to study eomysticetid fossils from the south island of New Zealand. Eomysticetids are a thus far poorly known group of early baleen whales, and constitute the earliest known and earliest diverging toothless baleen whales. So far, the only eomysticetids that have been described include Eomysticetus whitmorei and Eomysticetus carolinensis from the Oligocene of South Carolina, described by Larry Barnes and Al Sanders in 2002 in the Clayton Ray memorial volume. However, in that same volume, Barnes and Sanders name another new family of early diverging mysticetes they term the Micromysticetidae; they remove Cetotheriopsis tobieni from said genus and place it in the new genus Micromysticetus, to which they also name a new species from South Carolina, Cetotheriopsis rothauseni. This family also includes the taxon Cetotheriopsis lintianus. Anyway, Micromysticetus has almost always occurred as a sister taxon to Eomysticetus wherever included in phylogenetic analyses, and I would not be surprised if the Eomysticetidae were to include these even smaller taxa.


The holotype skull of Eomysticetus whitmorei from South Carolina (borrowed from the morphobank account for Ekdale et al., 2011).

The new material from New Zealand includes a collection of eight partial and complete crania, many with dentaries, earbones, and postcrania. In addition, two species of Mauicetus may be referable to the Eomysticetidae, and part of this project will revolve around trying to ascertain whether any of these new specimens represents referable material of Mauicetus; the skulls of the two holotypes of two Mauicetus species (not including Mauicetus parki, which is not an eomysticetid) are very incomplete or have been lost, but are still known from some earbones and postcrania (and photos of the skulls). One of my tasks will almost certainly be to determine whether or not any of this new material could be designated as a neotype specimen.


The clocktower at University of Otago.

All of that interesting paleocetaceanology aside, Sarah and I are going to New Zealand!!! We'll be living in the city of Dunedin on the south island. Above you can see a photo of the clock tower at the university; the campus there looks absolutely beautiful. Granted, Traphagen Hall at MSU Bozeman is a neat old building (but totally shitty inside), but I've seen photos of the Geology Building at OU, and it looks just like another Tudor stone castle like the main building pictured above. It looks totally awesome. Furthermore, unlike my previous 8 years of schooling in Montana, it doesn't get anywhere near as cold on the south island (although Dunedin is about as far south as you can get on the south island). And lastly, there are penguins that live there! There are penguins that have rookeries on the Otago Peninsula, within a 30 minute drive from campus! Blue/Fairy penguins, the smallest known species of penguin!

This is going to be a blast, and I have a lot of work to do to get there.

Thursday, September 1, 2011

Recent fieldwork in the Purisima Formation, Part 3: mysticete earbones and wildlife

Hey Folks,

Sorry for yet another delay - I've been pretty busy, working on several manuscripts (a thesis-length paper on the Purisima Formation marine mammals from my undergraduate field area in Halfmoon Bay, a new manuscript on shark bitten cetacean bones, and my contribution to a paper of the mollusk and vertebrate assemblage of a late Miocene marine locality in Sonoma County), applying to the University of Otago Doctoral Program to work with R. Ewan Fordyce (in New Zealand), and digging up a new right whale fossil from the Purisima Formation. There are plenty of topics I have thought of to write about on here, but not enough time!


Continuing on with my series of posts about recent Purisima Fm. fieldwork with Dick Hilton, I've written a little about a new mysticete earbone. There are lots of mysticete earbones from the Purisima Fm., from number of different taxa, including cetotheriids, many balaenopterids, and balaenids. Dick had originally spotted this specimen during a field trip earlier in the spring, but was unable to collect it. On our first day of our expedition back in late May, we spotted it easily, and given the easier tides, we were able to quickly excavate it. I was immediately struck with the size of the specimen, and in particular a large knob called the dorsal posterior prominence. This very distinctive earbone morphology is characteristic of the extinct rorqual "Megaptera" miocaena, which Remington Kellogg described in the 1920's from the late Miocene Sisquoc Formation of southern California. Several authors including Deméré et al. (2005) and Dooley et al. (2004) have suggested that it does not belong in Megaptera at all, and that it requires a new genus to be erected. However, it has appeared in some phylogenetic analyses (Bisconti, 2008; Marx, 2010) as a sister taxon to modern Megaptera novaeangliae (the modern Humpback Whale for the uninitiated). It really needs to be reanalyzed and probably redescribed.


Fossil tympanics of "Megaptera" miocaena from the upper Miocene San Mateo Formation (left) and Purisima Formation (right).

Fossils of this taxon are now known from Tortonian and Messinian (6-11 Million Years Old) strata in California, including the Sisquoc Formation, Purisima Formation (two localities), and the Santa Margarita Sandstone (a new specimen of which will soon be donated to UCMP). Other vertebrates from this time period include the dusignathine walruses Pontolis and Gomphotaria, the odontocetes Denebola, Parapontoporia, Albireo, and Piscolithax, as well as other mysticetes such as Nannocetus and Herpetocetus; all of these taxa are now known from multiple strata of this age, suggesting a distinct, and well-represented late Miocene marine mammal fauna from the eastern North Pacific.

Lastly, we spotted some wildlife during the trip, the photos of which are below.


Northern elephant seals spotted from the point.

A peregrine falcon near a nest at the edge of a cliff.


A coyote that ran along the beach while we stopped for a snack.

References:

Bisconti, M. 2008. Morphology and phylogenetic relationships of a new eschrichtiid genus (Cetacea: Mysticeti) from the Early Pliocene of northern Italy. Biol J Linn Soc 153: 161–186.

Deméré, T.A., A. Berta, and M.R. McGowan. 2005. The taxonomic and evolutionary history of fossil and modern balaenopteroid mysticetes. Journal of Mammalian Evolution 12:99–143.

Dooley, A. C., Jr., Fraser, N. C., and Luo, Z.-X. 2004. The earliest known member of the rorqual-gray whale clade (Mammalia, Cetacea). J. Vertebr. Paleontol. 24: 453–463.

Kellogg, R. 1922. Description of the skull of Megaptera miocaena, a fossil humpback whale from the Miocene diatomaceous earth of Lompoc, California. Proc. US Natl. Mus. 61: 1–18.

Marx, F. G. 2010. The more the merrier? A large cladistic analysis of mysticetes,
and comments on the transition from teeth to baleen. J Mammal Evol 18:
77–100.

Tuesday, August 9, 2011

Recent fieldwork in the Purisima Formation, Part 2: a possible new species of Herpetocetus?

Back in late May, Dick Hilton (Sierra College) and I did a three day field trip collecting fossil vertebrates from a locality in the Purisima Formation I recently got a permit for. On the second day, excavated a large block of sediment with what I assumed at the time were sirenian bones. I had not seen the bones except in cross section, and because they were somewhat dense, I thought they might be from a sea cow. We quickly carved out a large block, and due to the cohesive nature of the sediment, we were able to wrap it in tinfoil and duct tape. It was one of the first finds of the day, and I thought there could definitely be something neat inside. Because we were only a half mile from the cars, I left my pack with Dick and hoofed it back to the car with the thirty pound block, and also to grab some gatorade I had left in my car. When I returned, Dick was taking a siesta, and after some lunch, we headed further down the beach. Only a few hundred feet down I spotted a distinctly potato-shaped thing sticking out next to a piece of bone: it rather looked to me like a tympanic bulla, and I climbed up a bit to check it out. It was in fact a tympanic, and when the rest of the piece came out, I was able to see that it was in fact a nearly complete squamosal, complete with the bulla and posterior process of the petrosal. Dick and I thought the trip had been a success just because of this specimen, especially because it was from a section of cliffs where neither of us expected to find anything.

Dick Hilton digging up a huge baleen whale tympanic.

I couldn't have been more wrong. Unfortunately, I didn't know that I was until after the SATLW (Aquatic Tetrapods) conference. I did have a day or two before the conference to prepare the squamosal, and it did indeed have a plug-shaped posterior process of the petrosal, indicating it belonged to the Herpetocetinae, which includes Herpetocetus, Nannocetus, (probably) Piscobalaena, and Cephalotropis (according to Steeman, 2007). After the conference, I opened up the duct taped jacket and began preparation. After a couple hours the exposed pieces were still not making sense, and then I found a couple of bones that looked like they were adjacent to one another. When I removed them, there was a tiny neck of bone connecting them – and after a little more preparation, I realized it was a Herpetocetus petrosal and posterior process. Damnit, another goddamn Herpetocetus.

The petrosal and posterior process of the new specimen, with the facial nerve canal labeled. Upper left is ventral, lower left is dorsal, and right is medial view.

The skull with (partially incorrectly) articulated petrosal of the new skull in dorsal (top) and ventral (bottom) views.

Once I had enough of the block prepared, I realized I had quite a bit of the ventral portion of a small braincase preserved. It includes both exoccipitals, one occipital condyle, the basioccipital, the right squamosal, and the complete petrosal. After preparation, the petrosal is most similar to petrosals of Herpetocetus. This may be a bit technical, but herpetocetine baleen whales have several peculiar features that define them as a group. The posterior process of the petrosal – which is typically an elongate strap of bone that connects with the skull posteriorly – is very short and plug-shaped in these animals. Additionally, the posterior process (which is rarely found attached in isolated fossil mysticete petrosals) is flat and contributes to the lateral side of the skull, instead of being 'hidden' in a trench between the squamosal and exoccipital bones. Secondly, some herpetocetines have a flattened anterior process that is blade shaped; this structure is typically conical and robust or knoblike in most other mysticetes. Clearly, this specimen exhibits both of these features. Additionally, Herpetocetus spp. exhibit a large triangular flange on the side of the bone, which overhangs the squamosal – also present in this specimen. Additionally, herpetocetines all have extremely small earbones relative to most mysticetes. Unfortunately, the neck of the posterior process appears to have been deformed slightly, and when the main portion is articulated correctly, the posterior process sits in its trough a little wonky, and when the posterior process is articulated correctly, the main portion doesn't articulate well.

The posterior process, squamosal, and tympanic of Herpetocetus bramblei.

The two alternate articulations of the petrosal showing correct articulation of the posterior process (left) and correct articulation of the body of the petrosal (right).

The temporal region of the skull of Herpetocetus bramblei with the petrosal outlined in red.

However – it shows several features that differentiate it from all species of Herpetocetus as well as other herpetocetines like Nannocetus and Piscobalaena. Firstly, the anterior process is medially oriented – it is usually anteriorly facing instead. Second, the posterior process is very transversely narrow and elongate – it is typically more nearly circular in other species. Lastly, the most bizarre feature is that it has a very long anterior fissure of the facial nerve canal which is contorted into an S-shape – something I have not seen in any mysticete, fossil or modern.

Various mysticete petrosals in ventral view, showing two fossil rorquals (Plesiobalaenoptera and Balaenoptera sursiplana), a modern balaenid (Eubalaena japonica), the new specimen, and two other Herpetocetus specimens.

This is pretty exciting, and I am looking forward to preparing the other specimen, which includes part of a squamosal and a tympanic, and most likely a petrosal. It should not be too difficult to get these specimens written up and described.

Further Reading

Geisler, J. H. & Luo, Z.-X. 1996. The petrosal and inner ear of Herpetocetus sp. (Mammalia: Cetacea) and their implications for the phylogeny and hearing of archaic mysticetes. Journal of Vertebrate Paleontology, 70, 1045–1066.

Steeman, M.E. 2007. Cladistic analysis and a revised classification of fossil and recent mysticetes. Zoological Journal of the Linnean Society 150:875–894.

Steeman, M.E. 2010. The extinct baleen whale fauna from the Miocene-Pliocene of Belgium and the diagnostic cetacean ear bones. Journal of Systematic Palaeontology 8:63-80.

Whitmore, F.C., and L.G. Barnes. 2008. The Herpetocetinae, a new subfamily of extinct baleen whales (Mammalia, Cetacea, Cetotheriidae). In C.E. Ray, D.J. Bohaska, I.A. Koretsky, L.W. Ward, and L.G. Barnes (eds.). Geology and Paleontology of the Lee Creek Mine, North Carolina, IV. Virginia Museum of Natural History Special Publication 14:141–180.

Sunday, August 7, 2011

Recent fieldwork in the Purisima Formation, Part 1: Gigantor whale jaw

If you pay attention to paleo-related news on the intertubes, you may have seen a recent article about a 700 lb dinosaur bone excavated from the Morrison Formation near Fruita, Colorado. Fellow MSU student Krista Brundridge was even interviewed and involved in the excavation. They only state that the bone is from the animal's back, so I can only assume that it's a huge sauropod vertebra. Which means that maybe the kind folks over at SV-POW! will be drooling over the news. If people really wanted to dig up humongously sized plaster jackets, they'd come to California and dig up whales. Why, back in may, Dick Hilton and I prospected a locality in the Purisima that hasn't been collected by paleontologists in over twenty years, and over the course of two days, found dozens of multi-ton blocks just sitting there on the beach. Many of them had vertebrae (which unlike those of sauropods, are much more conservative in their anatomy), ribs, and other odds and ends. However, I counted many that had skulls. One block that was the size of a pickup truck had a complete skull, at least one lower jaw, and apparently part of an articulated vertebral column and ribcage.

Me posing with half of a gigantic whale jaw.

Wait a second, you say. Dinosaur paleontologists scrounge up every scrap of bone, and re-re-describe old fossils (i.e. Dryptosaurus was first described, then re-described, and then re-re-described), and bitch and moan about there not being enough material for new researchers. How would complete skulls of baleen whales just sit on the beach without some intrepid explorer to come along and excavate or collect them? Below, I've got a photo of what used to be a complete baleen whale jaw sitting in a large boulder, ~20 feet above the beach. I climbed up to it, which was pretty hairy – usually the Purisima Formation is sandstone, and easy to carve handholds in, but this was nasty hard fractured mudrock. This jaw must be in a concretion that weighs the same as my small Honda. For baleen whales, jaws are "relatively" diagnostic (see here, here, and Boessenecker 2011), so specimens like this are of interest. Baleen whale skulls are of course diagnostic, and it is unfortunate that they are languishing like this.

It was kind of a pain to get down from there.

One problem, you might say, is that they're big, and in very tough rock. Yes, I spent five years of my life (intermittently) preparing a mysticete skull in a concretion that I collected from the Purisima Formation. Sure, it's a big heavy skull, but surely smaller and less heavy than any ceratopsid skull you can point at. Obviously, blue whales have bigger crania than dinosaurs like Triceratops. Most fossil mysticetes have skulls that are smaller than or roughly the same length as the largest "Torosaurus" skulls, but many museums out there don't hesitate to go dig up more Triceratops skulls. Is it the often concretionary matrix and the time-intensive nature of the preparation that makes whale fossils "unpopular"? I don't think so, because I can't count the number of dinosaur bones (even undiagnostic material like ribs) encased in hard rock being prepared.

Permanently borrowed from SV-POW! Thanks guys, this image is awesome.

Are whales and whale fossils just unpopular within vertebrate paleontology? Maybe. Given how whales captivate the imagination – mind you, not in the gory, Velociraptor-chasing-kids-through-a-kitchen and lawyer-eating sort of way but the holy-shit-its-a-brachiosaurus-on-a-grassy-hill sort of way – I highly doubt that cetaceans lack the cool-factor. They may not have big sharp pointy teeth... oh shit, I forgot that fossil sperm whales are far more impressive than any puny theropod. Sorry, Livyatan beats T. rex. I think the real problem is that we have the Jurassic Park generation in vertebrate paloentology now – and not to sound like a bitchy hipster, although I am of the correct age group – I was into paleontology before Jurassic Park came out.

Nevermind that in the background.

Perhaps this is a problem that is, within the United States, unique to Northern and Central California. Southern California fossil cetaceans are really well taken care of, and get excavated and pampered at places like LACM, the Cooper Center, and the San Diego Natural History Museum. The extremely rich Calvert Cliffs and other Mio-Pliocene units of the Chesapeake Group of the mid Atlantic coastal plain are covered by the Calvert Marine Museum, the Smithsonian, and my dear friend Butch Dooley at the Virginia Museum of Natural History. Florida fossils are generally covered by the FLMNH and the University of Florida. The comparatively rich fossil record in the Oligocene and Miocene of Washington State (and parts of Oregon as well) are covered by the Burke Museum in Seattle. However, all of the UCMP students who collected a ton of material from Northern California in the 1970's and early 1980's moved on elsewhere.

I don't mean to complain – having a surplus of fossils available for my research is nothing to complain about. However, it is depressing if not distressing to see so many fossils I could not collect, prepare, and study alone in five or six lifetimes, just sitting out there on the beach. So: to all of you dinosaur folks who feel perhaps the field is a little too crowded, too much of a circlejerk, or whatever, come join marine mammal paleontology! Trust me, there are is a large hoard of new genera and species out there just waiting for the taxonomically hungry. In five years of serious collecting, I've got enough material to research for another ten years, and this is barely scraping the surface. So, this is a call for action! If you're interested in marine mammal paleontology, go dig up a whale (instead of Apatosaurus #32, or NewGenusOfUninterestingChineseDinoBird #54, or re-re-redescribing something everyone is already familiar with) or find someone who can help you (...or me, for that matter).

Unfortunately, the sad reality is that that jaw I posted above will probably not be collected. I don't have the funding, resources, or the connections (read: friends with heavy machinery) to collect stuff like that now. To be honest, it isn't complete enough for it to be worth it anyway. But that's besides the point: it was at one point, and another one will come along that will be worth collecting. Will we be up to the challenge?

Sorry for the rambling here, the rest of these posts will be about fieldwork I did with Dick Hilton in May, I promise!

Tuesday, August 2, 2011

More problems with Herpetocetus

Back in June at the Aquatic Tetrapods conference I coauthored a poster with Joe El Adli (San Diego Natural History Museum) and Jonathan Geisler (New York College of Osteopathic Medicine) on some of the taxonomic problems of Herpetocetus. Herpetocetus, as I've mentioned before, is an enigmatic small bodied mysticete whale which many bizarre and derived features, while retaining some primitive features as well. Fossils of Herpetocetus are fairly common in Northern California, particularly in the Purisima Formation - or maybe I just have a knack for finding them. Thus far, there is only one described species of Herpetocetus from California: Herpetocetus bramblei, named by Whitmore and Barnes (2008) from a very partial skull (basically just a squamosal with part of the exoccipital, parietal, and pterygoid) with a petrosal from the Purisima Formation. In summer 2007, I excavated a nearly complete skull of this same species from near the type locality, and last summer, I excavated a second specimen which lacked the braincase but included a complete rostrum. Since this topotypic material was collected, additional specimens from other localities in the Purisima Formation indicate that two additional undescribed species are present - one of the new species was discovered very recently, and I'll have more on that soon.

*Holotype, for the non-specialist, is the specimen which a new species is based off of. It should be representative of the new species in terms of its anatomy, and should be relatively complete enough to be comparable to other taxa. A type locality is where the holotype specimen originated.

There are several other described species of Herpetocetus from other corners of the globe - all from the Northern Hemisphere. The genus was first described from the Pliocene of Belgium (Herpetocetus scaldiensis) based on a partial dentary. A partial skull from the Pliocene Yorktown Formation was described as Herpetocetus transatlanticus, also by Whitmore and Barnes (2008). In the 1960's, an isolated tympanic bulla from Japan was named as the type specimen of Mitzuhoptera sendaicus, and a fossil mysticete skeleton with a skull, earbones, and dentary shared both the dentary morphology of Herpetocetus scaldiensis as well as the tympanic morphology of Mitzuhoptera sendaicus, and Oishi and Hasegawa (1995) transferred M. sendaicus to Herpetocetus, resulting in the new combination, Herpetocetus sendaicus. Each of these records is from either side of the Pacific (east and west) and the Atlantic (east and west).

How diagnostic are bullae and dentaries? I've already addressed problems with the jaw morphology of herpetocetines (here and here), and mysticetes in general. If you recall, there are two problems concerning the dentary of Herpetocetus spp. in particular: 1) The dentary of the possible sister taxon Nannocetus is not yet known, and dentaries substantially older than Herpetocetus (and possibly belonging to Nannocetus) are nearly identical to Herpetocetus (see below image), indicating that this general morphology is possibly characteristic of a larger group of whales. 2) Some species of Herpetocetus have dentaries that are very difficult to tell apart and lack autapomorphic characters (unique derived features), and thus are not suitable as holotypes. This logically results in the implication that Herpetocetus scaldiensis, which is based on a jaw, is the type species of Herpetocetus, and thus the species and genus may be taxonomically invalid or nomina dubia (means dubious name in latin).

The first figure of our poster, showing comparative drawings of various fossil herpetocetines.

Earbones have long been used for taxonomic purposes, and in many cases have been designated as holotypes. Sir Richard Owen designated many isolated bullae from the Plio-Pleistocene Red Crag of eastern England as holotypes (all of which have been sunk; e.g. Balaena definata). It is unclear how diagnostic earbones are for baleen whales: petrosals (otherwise known as periotics - the inner ear bone) have all sorts holes and knobs and crests and are rather easy to tell apart from genus to genus. A recent paper published by Eric Ekdale, Annalisa Berta, and Tom Demere (2011) indicate that earbones of extant mysticetes are diagnostic to the species and are easily told apart. Additionally, Steeman (2010) reexamined a large suite of earbones previously described by taxonomic mad man P.J. Van Beneden, who is largely responsible for constipating the entire field of mysticete systematics for over 100 years. Steeman (2010) found that many of these earbones - specifically petrosals - may be diagnostic tools, and generally reached a similar conclusion like Ekdale et al. (2011). But what about bullae?


The second figure from our poster, showing variation in tympanic bulla morphology from various herpetocetines. Note the overall similarity between Herpetocetus spp.

Bullae of three species of Herpetocetus have been described: H. scaldiensis, H. transatlanticus, and H. sendaicus. In our poster, we figured all known bullae (described or undescribed), including both the holotype of Mizuhoptera sendaicus and the referred specimen of Herpetocetus sendaicus, and a new bulla of Herpetocetus bramblei. Additionally figured are bullae of Nannocetus and Piscobalaena, also herpetocetines. We concluded, as we hope that you will when looking at this figure, that the bullae of different Herpetocetus species do not vary significantly from species to species. They are, on the other hand, diagnostic at the family level: they are clearly distinct from all other bullae of (described) cetotheriids. However, a bulla that is only distinct at the genus level is inadequate to be used as a holotype. This suggests that Mizuhoptera sendaicus, unsurprisingly, is probably a nomen dubium. It also indicates something interesting is going on with the skulls of mysticetes, or at least cetotheriids: tympanics are slightly less informative than the petrosals. It might be possible someday to quantify how phylogenetically useful different anatomical regions are, aside from just counting up the number of characters used per anatomic region in a cladistic analysis. Who knows, maybe someone has already thought of that and developed a method.

Further Reading:

New published article (Part 1): herpetocetine jaws, and an example of finding a "simple" research project


New published article (Part 2): taxonomic problems with Herpetocetus and "cetotheres"

References:


El Adli, J., Boessenecker, R.W., and J. H. Geisler. 2011. Taxonomic problems of and relationships among species of the fossil baleen whale genus Herpetocetus. Sixth Triennial Conference on Secondary Adaptation of Tetrapods to Life in Water Program with Abstracts: 23.

Ekdale, E.G., A. Berta, and T.A. Demere. 2011. The comparative osteology of the petrotympanic complex (ear region) of extant baleen whales (Cetacea: Mysticeti). PLOS One 6:1-42.

Oishi, M., and Y. Hasegawa 1995. Diversity of Pliocene mysticetes from eastern Japan. The Island Arc 3:436–552.

Steeman, M.E. 2010. The extinct baleen whale fauna from the Miocene-Pliocene of Belgium and the diagnostic cetacean ear bones. Journal of Systematic Palaeontology 8:1:63-80.

Whitmore, F.C., and L.G. Barnes. 2008. The Herpetocetinae, a new subfamily of extinct baleen whales (Mammalia, Cetacea, Cetotheriidae). In C.E. Ray, D.J. Bohaska, I.A. Koretsky, L.W. Ward, and L.G. Barnes (eds.). Geology and Paleontology of the Lee Creek Mine, North Carolina, IV. Virginia Museum of Natural History Special Publication 14:141–180.

Tuesday, June 21, 2011

Sixth Triennial conference on the Secondary Adaptation of Tetrapods to Life in the Water

Two weeks ago today, I delivered a presentation on the first day of the 2011 Aquatic Tetrapods conference in beautiful San Diego, California. I had eight hours on my drive down to San Diego the day before to worry about how screwed I was: the last time I gave that presentation, it was only 20 slides longer, and took 50 minutes to deliver. I practiced it once Monday morning in front of Joe El Adli (our gracious host), and Yale students Rachel Racicot and Daniel Field - I barely fit it into 20 minutes. It all worked out fine, and in the actual presentation, I finished the last conclusion slide right as it counted down to zero. This was a fresh break from SVP tradition, which dicates that cetacean research is presented on the afternoon of the last day, giving you all week to worry about the presentation. This time, I was able to relax during the entire meeting.

My title slide for my taphonomy presentation.

It would be very difficult to summarize all the research presented, but I might be able to summarize a few of the highlights that stick out in my mind. Julia Fahlke (University of Michigan) gave a fascinating talk Monday Morning about basilosaurid and protocetid cetaceans with asymmetrical crania, and implications for the evolution of hearing underwater. I'll admit, when I read the abstract I was skeptical, but her presentation was pretty compelling - I'll wait to say more until it gets published, though. Brian Beatty presented some details of his research on meningeal ossification in cetacea, which appears to not be homologous to that in many other mammals. Larry Barnes showed us a new Paleoparadoxia skeleton the LACM has been working on from the Monterey Formation; it's virtually complete, with a very large, gnarly looking skull. Olivier Lambert gave a talk coauthored by Giovanni Bianucci on a new large assemblage of bizarre ziphiid fossils dredged from the seafloor off the coast of Spain; boy, there are some real freaks. Our Australian colleague Erich Fitzgerald presented a new juvenile aetiocetid skull from the Oligocene of Washington State which he's been slowly preparing with acid; needless to say, it's a beautiful specimen. Manuel Martinez, a Peruvian who is Christian de Muizon's Ph.D. student, presented on an incredible new toothed mysticete from the Oligocene of Peru - I won't give any details, but lets just say this will be a very, very important specimen.
Frank Fish gives a mini presentation on locomotor adaptations of various marine mammals, using an assortment of articulated limbs (a walrus forelimb is seen in the foreground).

On wednesday, we went over to the San Diego Natural History Museum for an osteology workshop on aquatic tetrapods. Due to the research focus of Tom Demere (Paleo curator) and Annalisa Berta, the majority of material out on display was from modern and fossil marine mammals. There was a great assortment of wonderful stuff out, and it was amazing to be there with so many other marine mammal (and otherwise) researchers there.

Several cetacean researchers are in this photo: Toshiyuki Kimura (foreground), Mette Steeman (behind "Tosh"), and Giovanni Bianucci (background, left) and Joe El Adli (background, right).

At the workshop, I caught Brian Beatty red-handed demonstrating his very technical method to determine the relative height of the bony tentorium (here on a skull of the Amazon river dolphin, Inia geoffrensis).


For a while, Daryl Domning gave a short presentation on the locomotion and forelimb of sirenians (using a Manatee forelimb skeleton).

Here, some of the brightest minds in cetacean paleontology scrutinize one of the weirdest fossil mysticetes: a new species of Herpetocetus under study by Joe El Adli. From left to right: Mette Steeman, Joe El Adli (standing), Felix Marx (leaning over skull), Meredith Rivin (background), Giovanni Bianucci (in glasses), and Olivier Lambert (in red).

Manuel Martinez, a Peruvian researcher studying with Christian de Muizon in Paris, did not waste a chance to photobomb. Here he is photographed with a cast of the skull of the bizarre extinct edentulous* walrus Valenictus chulavistensis.

Daryl Domning again gives a short presentation, this time on sirenian crania. Here he is showing a cast of the skull of the world's largest sirenian, the extinct Pliocene species Hydrodamalis cuestae (the ancestor of the "modern" Steller's Sea Cow).

My (soon to be) coauthor Morgan Churchill photographs an articulated hindlimb of the modern walrus.
Rachel Racicot (and Daniel Field) hung out with me for a bit in the type room at the San Diego Natural History museum while I photographed some fossil pinniped material. Skulls of gigantic Hydrodamalis cuestae sit on the table behind Rachel.